ES
 EN
 DE

A research-focused comparison of Melanotan II and PT-141, covering melanocortin receptor selectivity, evidence, safety signals and regulatory status.
This article is for educational purposes only and presents the state of scientific knowledge on mitochondrial biology and the processes of ageing. It does not constitute medical advice or a recommendation to use any substances. The compounds mentioned are described as objects of research, not as products for human use.
Mitochondria are organelles that generate most of the cell’s ATP through oxidative phosphorylation. Mitochondrial dysfunction — a decline in oxidative capacity, an accumulation of damage and impaired quality control of these organelles — is one of the hallmarks of ageing described in the literature on the biology of ageing.
In the classical view, mitochondria act as the cell’s powerhouses. The respiratory chain in the inner mitochondrial membrane transfers electrons and builds a proton gradient, which ATP synthase uses to produce ATP — the energy carrier in the cell’s energy metabolism. This is a picture that made its way into textbooks and remains accurate.
Research over the past two decades has, however, revealed a second face of these organelles. Mitochondria also act as signalling hubs. They participate in the regulation of apoptosis, calcium homeostasis and in so-called retrograde signalling — the transmission of information from the mitochondrion to the cell nucleus, which modifies the expression of nuclear genes in response to the organelle’s energy status.
A separate category comprises mitochondrial-derived peptides (MDPs), such as MOTS-c and humanin. These are short peptides encoded within the mitochondrial DNA, studied as signalling molecules in the context of metabolism and the processes of ageing. Their discovery consolidated the view that the mitochondrion is not merely an energy generator but an element of a broader network of cellular communication.
This dual role matters for understanding ageing. If the mitochondrion conveys to the nucleus information about its energy status, then the age-related decline in its function does not remain a local matter — it alters the signals reaching the genome and influences broader cellular programmes. In the literature on the biology of ageing, mitochondria are for this reason sometimes described as a node integrating information about metabolism, stress and homeostasis, rather than as an isolated organelle.
Historically, one of the most frequently cited concepts is the mitochondrial free-radical theory of ageing, formulated by Denham Harman in the mid-twentieth century. In its original version, reactive oxygen species (ROS), arising as a by-product of the respiratory chain, were thought to progressively damage mtDNA, proteins and lipids, and the accumulation of this damage was thought to drive ageing.
The contemporary picture is, however, markedly more nuanced. ROS have turned out to be not only a damaging factor but also signalling molecules. The phenomenon termed mitohormesis describes a situation in which a moderate, transient rise in ROS levels triggers adaptive cellular responses. In this view, ROS act as a physiological signal, not solely as a poison.
A consequence of this shift in perspective is that the simple version of the hypothesis — “ROS equals ageing, and antioxidants equal youth” — has not been confirmed in interventional studies. Trials in which high doses of antioxidants were administered generally did not deliver the expected extension of lifespan in experimental models, and some analyses even signalled effects opposite to those intended. One of the proposed explanations is precisely mitohormesis: excessive suppression of the ROS signal may dampen the cell’s adaptive responses, which within a moderate range are beneficial.
It is worth emphasising that this is a report on an ongoing scientific debate, not a recommendation to use or to avoid antioxidant supplementation. The contemporary literature does not entirely reject the role of oxidative stress in ageing — rather, it shifts the emphasis from a simple balance of “free radicals versus antioxidants” to the question of the location, intensity and duration of the ROS signal and the cell’s capacity to respond to it. Oxidative damage remains a real phenomenon, yet its relationship with ageing has turned out to be more complex than the original hypothesis assumed.
Mitochondrial DNA (mtDNA) has features that make it particularly susceptible to damage. It is located physically close to the respiratory chain — and therefore close to the site where ROS are generated. Unlike nuclear DNA, mtDNA has a limited repertoire of repair mechanisms and is not protected by an elaborate histone structure.
As a result, with age an accumulation of mutations and deletions in mtDNA is observed in many tissues. Because each cell contains many copies of mtDNA, what matters is the proportion of mutated to normal copies (the phenomenon of heteroplasmy). When the share of mutated copies exceeds a certain threshold, it may translate into reduced efficiency of the respiratory chain in a given cell.
Studies on animal models with an elevated rate of mtDNA mutation — the so-called “mutator” mice, lacking effective proofreading of mitochondrial DNA replication — have linked this state with features of accelerated ageing. This is one of the arguments that moved mtDNA from the role of a passive witness to that of an active thread in the biology of ageing. There remains, however, a discussion as to what extent the age-related level of mtDNA mutation is, under physiological conditions, a cause and to what extent a consequence of, or a companion to, other processes. Regardless of how this debate is settled, the integrity of mtDNA remains one of the parameters describing the condition of mitochondria in the context of age.
The cell is not defenceless against the deteriorating state of mitochondria. It has at its disposal a network of quality-control mechanisms which, under conditions of health, maintain a pool of functional organelles.
These three processes — biogenesis, dynamics and mitophagy — do not operate in isolation but form a continuous cycle of renewal: damaged organelles are removed, and new ones arise in their place. The literature links a decline in the efficiency of this quality-control cycle with age, which favours the accumulation of damaged mitochondria and a reduction in the overall metabolic capacity of tissues. The connections between mitophagy and other pathways of cellular homeostasis maintenance are discussed more broadly in the article on autophagy, sirtuins and mTOR.
The state of mitochondria is closely interwoven with the energy metabolism of the entire cell, and one of the nodes of this interweaving is nicotinamide adenine dinucleotide (NAD+). NAD+ acts as a cofactor in the oxidation–reduction reactions of the respiratory chain and the Krebs cycle, transferring electrons and participating in the production of ATP.
NAD+ is at the same time a substrate for the sirtuins — a family of NAD+-dependent enzymes, some of which (for example SIRT3) localise to the mitochondria and participate in the regulation of their function. The literature describes a decline in the availability of NAD+ with age, which is sometimes linked with diminished sirtuin activity and changes in the functioning of mitochondria.
It is worth noting that these connections work in both directions. On the one hand, NAD+ powers the energy reactions within the mitochondrion; on the other, its pool in the cell depends on the balance between synthesis, consumption and recycling, in which NAD+-consuming enzymes are involved, such as the sirtuins or the PARP polymerases activated during the repair of damage. This creates a mitochondrial–metabolic axis linking the organelle’s energy status with cellular signalling, in which a decline in mitochondrial function and a fall in NAD+ availability may reinforce one another. NAD+ metabolism in the context of ageing is developed in a separate article on NAD+ and ageing.
Among the molecules studied at the intersection of mitochondrial biology and ageing is MOTS-c — a peptide encoded within mtDNA, classified among the mitochondrial-derived peptides. In the scientific literature it is described as a signalling molecule studied in the context of metabolism and energy homeostasis, which makes it an interesting object in this field.
MOTS-c as a substance is available on the market solely as a research reagent under the Research Use Only (RUO) regime. This means that it is a material intended for laboratory applications — RUO is neither a dietary supplement nor a product for human use, and this description serves as an educational bridge to the literature, not as a recommendation. The mechanism of action of MOTS-c and a detailed review of the research are discussed in a dedicated article, MOTS-c — a mitochondrial peptide in research; the reagent’s own datasheet can be found on the page for the MOTS-c 10 mg product.
The overview below signals directions of research in the area of mitochondrial biology and ageing. It is illustrative in character.
| Area | Model | Observation | Year | Source |
|---|---|---|---|---|
| Free-radical theory | theoretical framework | Formulation of the hypothesis of ROS as a factor in ageing | 1956 | Harman |
| Hallmarks of ageing | review | Mitochondrial dysfunction among the hallmarks of ageing | 2013 | López-Otín et al. |
| Mitophagy | cellular/animal models | The role of removing damaged mitochondria in homeostasis | review | Sun / Youle |
| mtDNA | animal models | Accumulation of mtDNA mutations and features of ageing | review | Wallace |
| Hallmarks update | review | Expanded account of the hallmarks of ageing | 2023 | López-Otín, Kroemer et al. |
What is mitochondrial dysfunction?
It is a general term for the reduced efficiency of mitochondria: a decline in oxidative capacity, an accumulation of damage to mtDNA and proteins, and impaired quality control of the organelles. In the literature on the biology of ageing it is counted among the hallmarks of ageing.
Do ROS really cause ageing?
The picture is nuanced. The original hypothesis treated ROS solely as a damaging factor, yet today it is known that they also play signalling roles (mitohormesis). The simple version of the theory and the efficacy of high doses of antioxidants have not been confirmed in interventional studies.
What is mitophagy?
Mitophagy is a selective form of autophagy in which the cell recognises and removes damaged mitochondria, directing them for degradation. A decline in its efficiency with age is thought to favour the accumulation of dysfunctional organelles.
How are mitochondria connected with NAD+?
NAD+ is a cofactor of the oxidation–reduction reactions in the respiratory chain and the Krebs cycle, as well as a substrate for the sirtuins, including the mitochondrial SIRT3. The decline in NAD+ availability with age described in the literature is sometimes linked with changes in mitochondrial function.
What is MOTS-c in the context of mitochondria?
MOTS-c is a mitochondrial-derived peptide, encoded within mtDNA, studied as a signalling molecule in metabolism. As a substance it remains an RUO research reagent. Details can be found in the dedicated article on MOTS-c.
Mitochondrial dysfunction is one of the hallmarks of ageing, tying together several threads of cell biology: the production of ATP, ROS signalling, the integrity of mtDNA and the mechanisms of quality control — biogenesis, dynamics and mitophagy. Contemporary research is moving away from the simple free-radical theory towards a picture in which the mitochondrion is both a powerhouse and a signalling node, interwoven with NAD+ metabolism and the pathways of homeostasis maintenance. Mitochondrial-derived peptides, such as MOTS-c, remain in this context an object of research interest — described here solely as an RUO reagent and a topic in the literature, not as a product for use. As across the whole longevity front, one principle applies here: the predominant part of the data comes from animal and cellular models, and a description of a mechanism is not equivalent to the existence of a confirmed intervention in humans.
The text above describes biological mechanisms and the state of scientific research. The substances mentioned, including MOTS-c, are research reagents under the Research Use Only regime and are neither dietary supplements nor products intended for human use. The article does not suggest the extension or rejuvenation of life, nor does it recommend the supplementation of antioxidants or any other substances. Any decisions concerning health should be consulted with a physician.
A research-focused comparison of Melanotan II and PT-141, covering melanocortin receptor selectivity, evidence, safety signals and regulatory status.
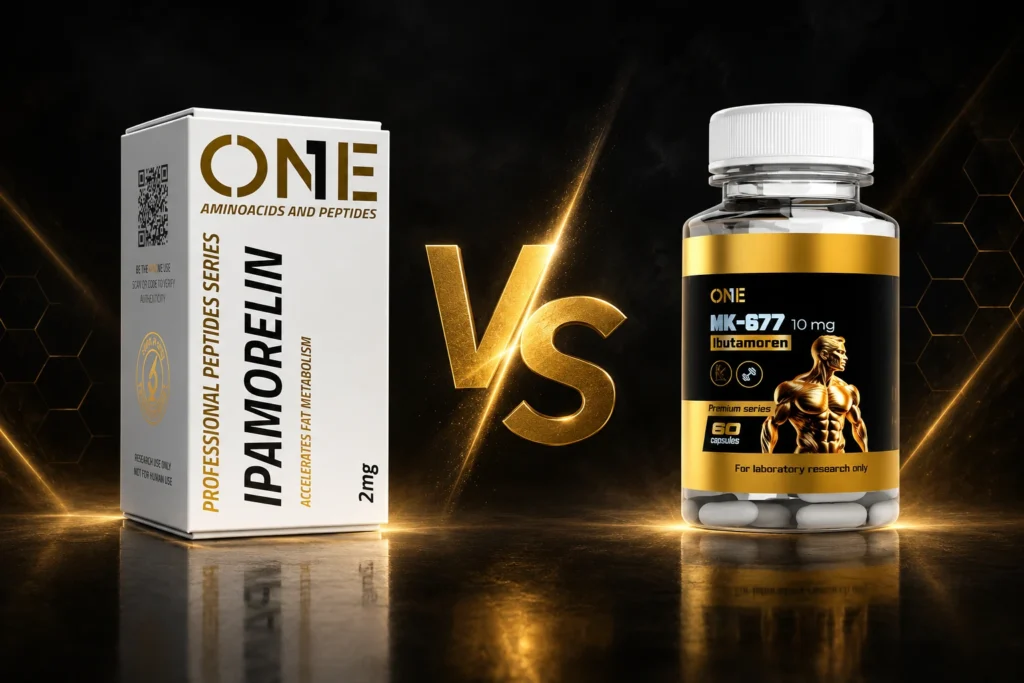
A research comparison of MK-677 and ipamorelin, focusing on GHS-R1a signaling, selectivity, administration route, human evidence and WADA status.