EN
 DE
 ES
 PL

A research-focused comparison of Melanotan II and PT-141, covering melanocortin receptor selectivity, evidence, safety signals and regulatory status.
This article is educational in nature and constitutes a review of the scientific literature on the molecular pathways studied in the biology of cellular ageing. It describes mechanisms at the level of enzymes, proteins and genes — it does not constitute medical or nutritional advice and does not contain any protocol, diet or instructions for use. Substances mentioned in the text are discussed solely within the framework of laboratory research.
Sirtuins, autophagy and mTOR are three molecular pathways that act within the cell like a network of sensors of its energy and nutrient status. Sirtuins read the level of the cofactor NAD+, mTOR senses the availability of building materials, and autophagy recycles the cell’s worn-out components. The biology of ageing studies this network as one of the organism’s central regulatory circuits.
Over the past two decades these three names — sirtuins, mTOR and autophagy — have become a foundation of the molecular biology of ageing. Not because anyone learned to “steer” them, but because studies on cells and animal models have shown how deeply these pathways are woven into the cell’s metabolism, repair and survival. This article describes what each of them is at the molecular level and how they combine into a single regulatory network — without venturing into what anyone might “do” with that knowledge.
Sirtuins are a family of seven enzymes (SIRT1–SIRT7) belonging to the class of deacetylases — proteins that remove acetyl groups from other proteins. The feature that makes them so interesting for the biology of ageing is this: sirtuins require the cofactor NAD+ to function (nicotinamide adenine dinucleotide). The deacetylation reaction consumes NAD+, so sirtuin activity is directly coupled to the availability of this cofactor within the cell.
In molecular practice this means that sirtuins act as a readout of the cell’s metabolic state. NAD+ is a central participant in energy reactions, and its pool changes together with metabolism. Sirtuins “sense” this level and translate it into modifications of regulatory proteins.
The family is not uniform. Individual sirtuins have different locations and targets:
Sirtuins do not “switch on youth” — they modify the activity of hundreds of target proteins, and the outcome depends on the cellular context. What links them to the longevity narrative is an observation from laboratory models: sirtuin activity is associated with the regulation of genes of the metabolic stress response and with mitochondrial function — two areas that change with the age of the cell.
Because sirtuin activity depends on NAD+, and the NAD+ pool in tissues declines with age, the two topics are closely linked in the literature. This thread is developed more fully in a separate article on NAD+ metabolism in the context of ageing, to which we refer as the biochemical background for the entire sirtuin family. NAD+ precursors, such as NMN, are studied as laboratory tools that modulate the pool of this cofactor ⚠️ (substances with RUO status, discussed for research purposes only).
mTOR (mechanistic target of rapamycin) is a kinase — an enzyme that attaches phosphate groups to other proteins — that serves within the cell as the principal sensor of nutrient availability and growth signals. The name derives from rapamycin, a compound isolated from a soil bacterium, which inhibits this kinase.
At the molecular level mTOR acts within two protein complexes: mTORC1 and mTORC2, with different functions and sensitivities. It is mTORC1 that is the main integrator of nutrient signals — it responds to the availability of amino acids, the cell’s energy state and growth-factor signals.
The logic of mTOR’s action is opposed to that of autophagy. When the cell has access to building materials, mTORC1 is active and directs the cell into growth mode: it intensifies protein synthesis, supports the construction of new structures and at the same time inhibits autophagy — because under conditions of abundance there is no need to break down its own components into parts. mTORC1 phosphorylates proteins that initiate autophagy (including ULK1), keeping this process in a switched-off state.
The inverse relationship is equally important: inhibiting mTOR unblocks autophagy. This is precisely why rapamycin — a pharmacological inhibitor of mTORC1 — has become one of the most frequently studied compounds in the biology of ageing. In animal models, mTOR inhibition has been associated with intensified autophagy and with phenotypic changes towards the slowing of certain processes of cellular ageing. The framing is worth emphasising: these are observations from laboratory and animal models, describing a mechanism, and not recommendations or established applications in humans.
If mTOR is a sensor of abundance, then AMPK (AMP-activated protein kinase) is its molecular mirror — a sensor of energy deficit. AMPK monitors the AMP/ATP ratio within the cell, that is, the balance of the “empty” and “charged” energy currency. When ATP is consumed faster than it is generated, the level of AMP rises and AMPK becomes activated.
Active AMPK switches the cell from build mode to a mode of energy conservation and recovery. At the molecular level it does this in two ways that tie together the entire circuit under discussion:
An opposing axis thus arises: AMPK↑ means mTOR↓, and together this leads to the unblocking of autophagy. This is an elegant example of a cellular switch — one sensor (abundance, mTOR) and another (deficit, AMPK) act in opposition on the same effector proteins. The mitochondrial peptide MOTS-c, described in a separate article in this series, is studied precisely as a molecule that activates AMPK — one of the points of contact between this network and the peptide literature.
Autophagy (from the Greek for “self-eating”) is a process in which the cell degrades and recycles its own components — damaged proteins, worn-out organelles, aggregates. This is not an emergency mechanism but a continuously operating system of quality control and material recovery. For deciphering its molecular machinery Yoshinori Ohsumi received the Nobel Prize in Physiology or Medicine in 2016.
The canonical course of autophagy (macroautophagy) is a molecular sequence:
The molecular role of autophagy in the biology of ageing arises from its housekeeping function. Removing damaged mitochondria (mitophagy) and misfolded proteins limits the accumulation of molecular “waste” that builds up in ageing cells. In laboratory models, the efficiency of the ATG machinery has been associated with better maintenance of protein homeostasis (proteostasis). Let us emphasise, however, the nature of this description: it is a mechanistic relationship observed in cells and model organisms, and not an instruction on how to induce or intensify this process in humans. This article describes what autophagy is, not how one might influence it.
The real explanatory value appears when, instead of three separate pathways, we look at a single network. Sirtuins, mTOR, AMPK and autophagy form a circuit of sensors of the cell’s energy and nutrient status, in which signals converge on shared effector proteins.
At the core of this network is the opposing pair of sensors. Under conditions of nutrient abundance mTORC1 is active, promotes synthesis and growth, and keeps autophagy switched off. Under conditions of energy deficit — recognised at the molecular level as a rise in the AMP/ATP ratio — AMPK is activated, which inhibits mTORC1 and unblocks autophagy. In other words: under energy deficit the axis shifts towards AMPK↑ / mTOR↓, which molecularly reveals the cellular recycling programme. This is biology observed in cells, the way the cell responds to its own energy balance — not a prescription for the organism.
Sirtuins slot into this circuit through metabolism. Their activity depends on NAD+, and the NAD+ level changes together with the energy state — the same one that AMPK reads. The literature also describes molecular loops linking the two sensors: AMPK can influence the NAD+ pool and thereby the activity of SIRT1, while SIRT1 deacetylates proteins that modulate metabolism and mitochondrial biogenesis. A network of mutual feedback thus arises, in which the energy signal, the nutrient signal and the redox signal (NAD+) meet at the regulation of gene expression and at the autophagy machinery.
This is why the biology of ageing treats these pathways together. These are not four independent levers but a single integrated system for measuring the cell’s state — and it is as such a system that it is studied in the context of the mechanisms of cellular ageing.
The table below organises the observations from the molecular and preclinical literature that are cited most often. All of them concern cellular or animal models and describe a mechanism — they do not constitute conclusions about application in humans.
| Area / pathway | Research model | Mechanistic observation | Year | Source |
|---|---|---|---|---|
| Autophagy — ATG machinery | Yeast, cells | Identification of the ATG genes and the molecular course of the autophagosome → lysosome pathway (foundation honoured with the Nobel Prize) | 1993–2016 | Ohsumi |
| mTOR — inhibition and lifespan | Mice | Pharmacological inhibition of mTOR (rapamycin) was associated with an extension of median lifespan in a mouse model | 2009 | Harrison |
| Sirtuins — NAD+ and gene regulation | Cells, animal models | SIRT1 as an NAD+-dependent deacetylase regulating the expression of metabolic and stress-response genes | 2000–2013 | Guarente |
| Autophagy and cellular ageing | Review, models | The role of autophagy in maintaining proteostasis and removing damaged organelles in the context of cell age | 2011 | Mizushima |
| mTOR as a node of ageing | Review | Integration of nutrient signals by mTOR as a mechanism linking metabolism with ageing | 2013 | Johnson |
The common denominator of these works is this: they describe a mechanism, and the strongest phenotypic data (for example, the effect of mTOR inhibition on lifespan) come from animal models. Translation to human biology remains a separate, open research question.
What are sirtuins?
Sirtuins are a family of seven enzymes (SIRT1–SIRT7) of the deacetylase class, which remove acetyl groups from target proteins. Their distinguishing feature is their dependence on the cofactor NAD+ — the reaction consumes NAD+, whereby sirtuin activity is coupled to the cell’s metabolic state. They regulate gene expression, metabolism and the stress response.
What is autophagy?
Autophagy is a molecular process in which the cell degrades and recycles its own components. Damaged proteins and organelles become surrounded by a membrane (the autophagosome), which then merges with the lysosome, where the contents are broken down into building blocks that return to metabolism. It is a continuously operating system of quality control of the cell’s interior, described at the level of the ATG genes — not an event that this article teaches one to induce.
What does mTOR do?
mTOR is a kinase that serves as a sensor of nutrient availability and growth signals. When the cell has access to building materials, the mTORC1 complex is active, promotes protein synthesis and growth, and inhibits autophagy. Inhibiting mTOR (for example, through rapamycin in laboratory models) reverses this state and unblocks autophagy.
How do sirtuins connect with NAD+?
NAD+ is an obligatory cofactor of the reaction catalysed by sirtuins — without it these enzymes do not function. Because the NAD+ pool depends on energy metabolism (and changes with the age of the cell), sirtuin activity reflects the redox and energy state of the cell. This relationship is described more fully in a separate article on NAD+ metabolism in the context of ageing.
Can these pathways be “activated”?
This question lies beyond the scope of this article. Sirtuins, mTOR, AMPK and autophagy are the subject of basic research on cell biology, and the text describes their molecular mechanism — not methods of influencing them. The article does not contain and does not suggest any protocols, diets or procedures; any substances mentioned in the context of these pathways are discussed for research purposes only (RUO status).
Sirtuins, mTOR and autophagy are three pillars of the molecular biology of ageing which act within the cell like an integrated network of sensors of its energy and nutrient status. Sirtuins (SIRT1–SIRT7) are NAD+-dependent deacetylases linking metabolism with gene regulation. mTOR is a kinase-sensor of abundance, which promotes growth and inhibits autophagy. AMPK is its counterweight — a sensor of energy deficit, which inhibits mTOR and unblocks autophagy. Autophagy, in turn, is the machinery for the degradation and recycling of the cell’s components, described at the molecular level thanks to work honoured with the Nobel Prize in 2016.
The strongest data on the influence of these pathways on lifespan come from cellular and animal models and describe a mechanism, not an application. This is biology observed in the laboratory — the way in which the cell reads and integrates signals about its state. Understanding this circuit is a foundation of contemporary ageing biology; it is not, however, a set of instructions for use.
This article describes the molecular mechanisms of the sirtuin, mTOR, AMPK and autophagy pathways on the basis of the scientific and preclinical literature. It does not constitute medical or nutritional advice, and does not contain any protocol, diet or instructions for use. Substances mentioned in the text (for example, NAD+ precursors, mitochondrial peptides, rapamycin) are discussed solely within the framework of laboratory research and have the status of materials for scientific research (RUO). The text does not refer to the extension of life or rejuvenation in humans and does not make any health claims.
A research-focused comparison of Melanotan II and PT-141, covering melanocortin receptor selectivity, evidence, safety signals and regulatory status.
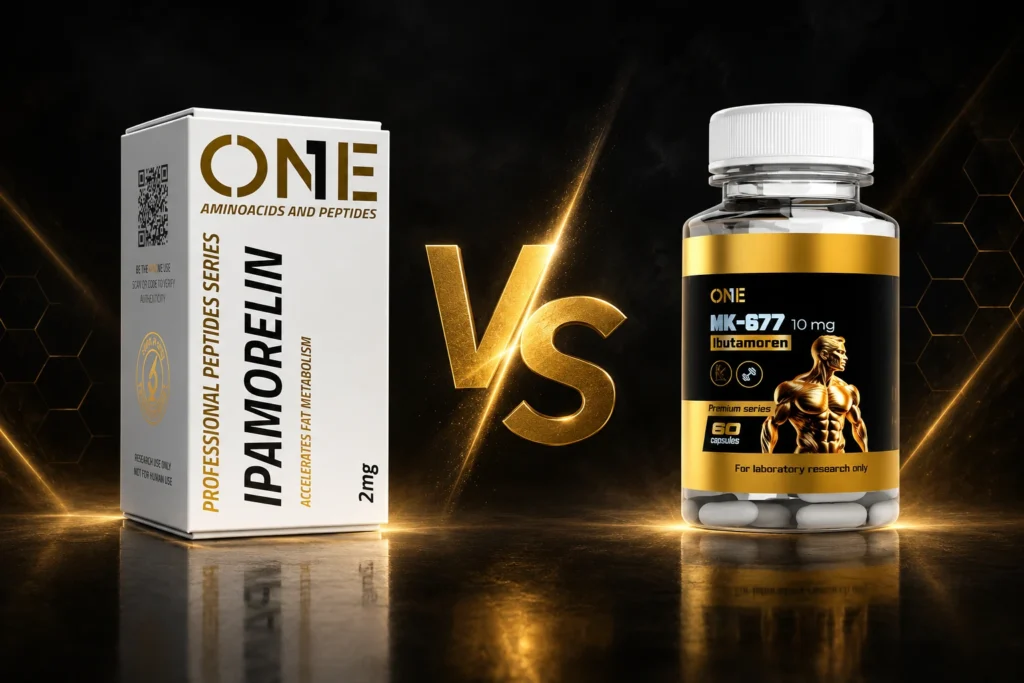
A research comparison of MK-677 and ipamorelin, focusing on GHS-R1a signaling, selectivity, administration route, human evidence and WADA status.